The useful comparison is by job.
Skin structure is a collaboration between fibres, cell attachments and signalling molecules. The four names in the earlier Replexium account belong to different parts of that collaboration. A change in one cannot substitute for measurements of the others.
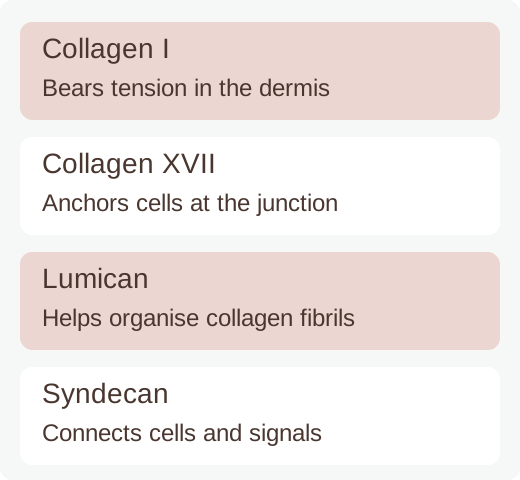
Collagen I: the tensile framework.
Type I collagen is a major fibre-forming collagen in skin, tendon and bone. Its precursor chains undergo hydroxylation and other modifications before they assemble into a triple helix. After secretion, the terminal propeptides are removed and the molecules gather into fibrils.
Lysyl oxidase helps stabilise those fibrils through cross-linking. Other matrix components control their size and arrangement. Collagen production, maturation and organisation are separate steps; a higher level of collagen messenger RNA measures only part of that process.
Turnover is regulated too. MMPs, or matrix metalloproteinases, cut collagen during normal remodelling and disease. Their inhibitors help balance breakdown. TGF-beta signalling influences production, but sustained activation can also contribute to fibrosis.
Collagen XVII: an anchor at the junction.
Collagen XVII spans the membrane of basal keratinocytes, cells at the bottom of the epidermis. It is part of hemidesmosomes: specialised attachment structures that help connect these cells to the basement membrane below.
Enzymes can shed its outer portion, changing the attachment and signalling environment. Research links collagen XVII with keratinocyte movement, epidermal stem-cell maintenance and skin homeostasis. Those functions differ from the load-bearing work of collagen I.
Lumican: organisation at the fibril.
Lumican is a small leucine-rich proteoglycan. Its protein core contains repeating structural regions, and its attached sugars vary by tissue. It interacts with collagen fibrils and helps regulate how they assemble and grow.
Genetic studies in mice with no lumican show abnormal collagen organisation, skin fragility and corneal changes. They establish the importance of the protein in those models; they do not establish the effect of a cosmetic ingredient said to increase it.
Lumican also participates in cell migration, inflammation and fibrosis-related signalling. Its effects depend on tissue and context, so “more lumican” is not a universal clinical endpoint.
Syndecans: the signal-bearing surface.
Syndecans are a family of cell-surface proteoglycans. Their outer sugar chains bind matrix components and signalling proteins. In this role they can act as co-receptors, helping present a signal to another receptor.
They cooperate with integrins in adhesion and movement. Syndecan-1 and syndecan-4 have different expression patterns and functions. Enzymatic shedding can release the outer domain into the surrounding matrix, changing how growth factors are held and presented.
The rest of the weave matters.
Elastin and fibrillin. Tropoelastin is the soluble precursor of elastin. Its assembly and cross-linking onto a microfibrillar scaffold create elastic fibres. Fibulin-5 and other partners help with this process. Damage to long-lived elastic fibres is a different problem from making new collagen.
Decorin, biglycan, aggrecan and perlecan. These proteoglycans contribute to fibre organisation, hydration, resistance to compression or basement-membrane function. Aggrecan is especially important in cartilage. Decorin also interacts with TGF-beta; perlecan helps hold growth factors locally.
Thrombospondin, SPARC and CCN2. These regulatory proteins influence cell adhesion, vessel growth, collagen assembly and fibrotic signalling. They illustrate why matrix biology is about control as well as material.
From protein biology to a research tool.
Researchers study matrix-derived peptides, recombinant proteins, small-molecule enzyme modulators, gene and cell approaches, and scaffolds designed to resemble the ECM. Laminin-derived sequences and the RGD cell-attachment motif are examples of using a small part of a larger structure in a biomaterial.
Each approach has tradeoffs. Broad MMP inhibition can interfere with useful processes. Collagen cross-linking enzymes also serve normal tissues. Delivery, immune responses, stability and off-target effects can all limit translation.
Imaging, proteomics and biomarkers of synthesis or breakdown may help test these ideas. Genetic differences can also affect matrix behaviour. Personalised treatment claims remain a larger step than identifying a plausible molecular target.
Reading boundary. The bibliography provides context for protein biology. It does not independently validate a commercial formulation.
Sources & further reading
Bibliography
- Trackman PC. Lysyl oxidase isoforms and potential therapeutic opportunities for fibrosis and cancer. Expert Opin Ther Targets . 2016;20(8):935-945. doi:10.1517/14728222.2016.1151003
- Ricard-Blum S, Vallet SD. Fragments generated upon extracellular matrix remodeling: Biological regulators and potential drugs. Matrix Biol . 2019;75-76:170-189. doi:10.1016/j.matbio.2017.11.005
- Natsuga K, Watanabe M, Nishie W, Shimizu H. Life before and beyond blistering: The role of collagen XVII in epidermal physiology. Exp Dermatol . 2019;28(10):1135-1141. doi:10.1111/exd.13550
- Liu N, Matsumura H, Kato T, et al. Stem cell competition orchestrates skin homeostasis and ageing. Nature . 2019;568(7752):344-350. doi:10.1038/s41586-019-1085-7
- Chakravarti S, Magnuson T, Lass JH, et al. Lumican regulates collagen fibril assembly: skin fragility and corneal opacity in the absence of lumican. J Cell Biol . 1998;141(5):1277-1286. doi:10.1083/jcb.141.5.1277
- Karamanou K, Franchi M, Vynios D, Brézillon S. Epithelial-to-mesenchymal transition and invadopodia markers in breast cancer: Lumican a key regulator. Semin Cancer Biol . 2020;62:125-133. doi:10.1016/j.semcancer.2019.08.003
- Couchman JR, Pataki CA. An introduction to proteoglycans and their localization. J Histochem Cytochem . 2012;60(12):885-897. doi:10.1369/0022155412464638
- Bass MD, Roach KA, Morgan MR, et al. Syndecan-4-dependent Rac1 regulation determines directional migration in response to the extracellular matrix. J Cell Biol . 2007;177(3):527-538. doi:10.1083/jcb.200610076
- Manon-Jensen T, Multhaupt HA, Couchman JR. Mapping of matrix metalloproteinase cleavage sites on syndecan-1 and syndecan-4 ectodomains. FEBS J . 2013;280(10):2320-2331. doi:10.1111/febs.12174
- Noda K, Dabovic B, Takagi K, et al. Latent TGF-β binding protein 4 promotes elastic fiber assembly by interacting with fibulin-5. Proc Natl Acad Sci USA . 2013;110(8):2852-2857. doi:10.1073/pnas.1215779110