Fibres, water and attachments.
The extracellular matrix is the material outside cells. In the dermis, collagen provides much of the resistance to pulling, while elastic fibres help tissue recoil. Long sugar chains called glycosaminoglycans, or GAGs, help hold water and give the matrix resistance to compression.
Proteoglycans combine a core protein with attached GAG chains. Decorin, biglycan, versican and perlecan have different organising and signalling roles. Hyaluronic acid is a GAG with an important distinction: it is not attached to a core protein.
The earlier edition’s general matrix and collagen reading is retained as PubMed record 27378178 and PubMed record 29186670.
Making collagen takes more than switching on a gene.
Fibroblasts first make precursor chains. Inside the cell, those chains undergo chemical modifications, including hydroxylation—adding hydroxyl groups—with vitamin C serving as a cofactor. The chains assemble into a triple helix and leave the cell as procollagen.
Outside the cell, enzymes remove the terminal propeptides so collagen can assemble into fibrils. Lysyl oxidase, a copper-dependent enzyme, helps create cross-links that stabilise the structure. Both too little organisation and abnormal cross-linking can impair its function. The earlier biosynthesis reference is PubMed record 22362372.
Fibrils gather into larger fibres. Their alignment, spacing and connections influence the mechanical behaviour of skin. A measurement of collagen quantity cannot fully describe that architecture; PubMed record 22995554 was the older edition’s link for this question.
Cells read their surroundings.
Integrins are cell-surface receptors that connect matrix proteins with the cell’s internal framework. Mechanical force through these connections can change signalling and gene expression. Cells alter the matrix, and the matrix alters the cells: a relationship often called dynamic reciprocity.
Proteoglycans also bind growth factors and influence where those signals are available. Perlecan is one example. Hyaluronic acid interacts with receptors such as CD44; fragment size and tissue context can change the response. The older hyaluronan link is PubMed record 21386386.
Matricellular proteins mainly regulate these interactions rather than acting as load-bearing fibres. Thrombospondin, SPARC and CCN proteins belong to this broader conversation. Their effects can differ between normal repair and chronic fibrosis. See the retained reading at PubMed record 25147176.
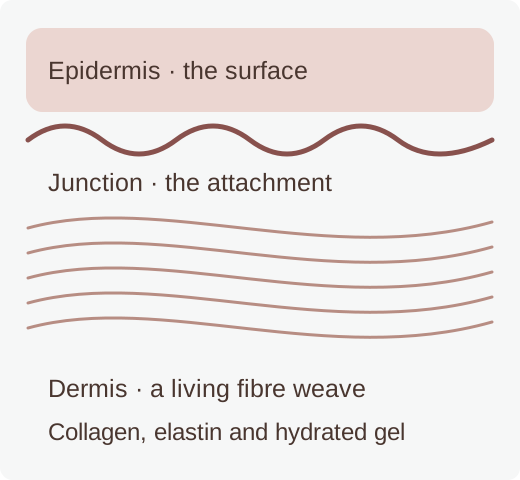
The surface has an attachment system.
The basement membrane is a specialised matrix beneath the epidermis. Type IV collagen and laminins help form its networks; other proteins connect it to neighbouring tissue. Type VII collagen forms anchoring fibrils, while collagen XVII participates in the cell-attachment machinery.
Elastic fibres have another assembly system, with elastin laid onto a microfibrillar scaffold that includes fibrillin. Their turnover and capacity for replacement differ from collagen’s. Treating all structural proteins as one “collagen pathway” misses these distinctions.
Ageing shifts the balance.
Matrix metalloproteinases, or MMPs, are enzymes that cut matrix components. They have useful roles in normal turnover and wound repair. Tissue inhibitors of metalloproteinases, or TIMPs, help regulate them. The goal in biology is controlled remodelling, not the complete elimination of degradation.
Ultraviolet exposure can increase damaging signalling and MMP activity. Glycation creates advanced glycation end products, or AGEs, which can alter cross-linking and matrix mechanics. Senescent cells—cells in a persistent growth-arrest state—can release inflammatory signals and enzymes, collectively called the senescence-associated secretory phenotype.
The earlier sources on UV-related damage and glycation remain PubMed record 20233013 and PubMed record 21810695. These processes overlap, but none is a complete explanation of ageing by itself.
Repair is a sequence, not a single switch.
Wound repair moves through clotting, inflammation, tissue formation and remodelling. A temporary fibrin and fibronectin matrix helps cells move into the wound. Later collagen deposition and reorganisation change strength and structure over time.
Too little matrix breakdown can obstruct useful remodelling; too much can impair closure. TGF-beta, a family of signalling proteins, influences both normal repair and fibrosis. Scar formation therefore cannot be understood simply as a lack of collagen. The earlier wound-repair reference is PubMed record 19040564.
What peptide studies try to change.
Studies of GHK-Cu, matrikines and other peptides examine matrix synthesis, inflammatory signalling, MMP regulation and cell behaviour. The retained copper-peptide reading is PubMed record 25530318. Changes in a culture or animal wound need human confirmation in the relevant formulation and route.
Ultrasound, optical coherence tomography and other imaging methods can help assess tissue architecture. Mechanical tests and surface measurements answer further questions. Delivery systems, engineered scaffolds and biomarker-guided research remain active areas, with important gaps between a plausible mechanism and a reliable clinical outcome.